Saturday, August 15, 2015


Friday, March 22, 2013
Great Science : It’s All About the Story

During
a recent meeting I had the pleasure of talking with Iain Patten, a professional
science writer in Europe. Iain travels
throughout Europe teaching scientists how to write high impact papers. We were very like minded about the scientific
process. I wanted to share some of information from our discussion here.
----------------------------------------------------------
Great,
high impact science papers tell an important new story with broad
implications. The story involves effort and planning from day one. Before you start experiments,
read and ask big questions.
· What are the potential stories that could
be told depending on the answers to your questions?
· What would be new and exciting about those
answers and where could they lead experimentally?
·
What are the different ways of telling the
story? Which ones are likely to be
exciting and which are not exciting?
You should have a clear idea of the potential stories when you start your project. Planning,
drafting and making figures with real data and imagined data must be a weekly activity. DO NOT gather data mindlessly and then try to
write a paper with everything in year 5….most people do this to some degree.
·
Make pretend figures of the result(s) that would
fit with your storyline and see what they might look like if they were really
convincing. This way you won’t forget
controls, you will have a clearer sense of the statistics you will use, and you
will think through the potential outcomes.
·
Constantly draft ‘pretend’ figures of results
describing alternative outcomes and think about where they might take you. This way you know where you could be headed
and you will be prepared. This will help
elevate the pressure to make the experimental result fit your hypothesis.
· Constantly reevaluating your story will reduce
wasted effort/experiments, help you maintain focus and set goals, and prevent
you from overlooking holes in your story or failing to complete experiments.
·
Remember that the story does not have to fit the
chronological order of the experiments.
Rearrange the work to tell the story.
· Plan, draft, make figures, see the best
experiments and storylines, do the experiments…repeat
High
impact scientists are journalists that gather evidence and assemble it into a
compelling story that changes how people think.
You must work on your story constantly.
It will light the path in front of you and the paper will be written as
you go.
·
When putting the final paper together, all that
matters is the data that tells the most compelling, clear and well-supported
story. You must be prepared to leave
things out and do more work that further supports the best story. This stuff happens near the end and it is the
toughest to accept when you are close to finishing.
·
Your conclusions must be supported by the data. Overstatement is the kiss of death from
editors.
·
As provided to me by an editor from Nature
Medicine, a great story often has the following components:
o Novel,
surprising, entertaining and broad implications/impact
o Strong
mechanistic insights
o In
vivo relevance
o Functional
manipulations
o Necessity
and sufficiency
o Elegance
·
Be clear about the core message of the
paper. If you can’t state the core
message in 10 words or less then you haven’t found the core message.
o Each
subheading and associated section of the paper builds logically toward the core
message
o Paragraphs
of each section have one message per paragraph and a logical transition from
one paragraph into the next. All working
to support the core message of the section.
o Plan
– draft – plan – draft…and repeat to get an elegant and clear message and structure
for the story.
·
Beware of stories that just connect existing
dots – the impact and advance tends to be small.
Think
carefully about the journal that fits your story best. A preliminary inquiry can save time. You must clearly (and without exaggeration)
explain how your article fits with the journal’s scope and what the core
message is and why it is novel and important.
o
The best reviewers are often experts outside of
your field. They can judge the technical
aspects of the work and assess the impact without the internal biases of the
field.
o
Editors recommend looking at the journal
editorial board for good reviewers to suggest.
These people have a reputation for solid, fair reviews. Exclude competitors.
Finally,
what are you reading for? It is good to
be an expert, but what you are really looking for is the following:
o
New and exciting plot lines for your story.
o
Gems of information that help you support and
tell your story.
o
New and exciting plot lines for future stories
(untold stories in waiting).
o
New and elegant techniques and approaches that
will help you tell a better story.
o
Literature that will confound your story and
contradict your interpretations/results.
o
Evidence that your story is novel and high
impact.
Good
luck!!! Have lots of ideas and chisel out the best stuff.
Sunday, February 17, 2013
The Epigenome Cometh

A
recent study by Liu and colleagues undertook an EWAS study of rheumatoid
arthritis (RA) to uncover DNA methylation changes that interact with genetic
factors to mediate disease risk. The
authors note that RA is an ideal test case for EWAS because the cell-types
involved (leukocytes) are well defined and easily isolated. In addition, the disease state can be ascertained
by measures of anti-citrullinated protein (CP) antibodies. The authors performed a genome-wide DNA
methylation analysis of whole blood from 354 rheumatoid arthritis patients and
335 healthy controls for which genome-wide SNP and CP antibody data were also
available. They first correct for
cellular heterogeneity in their blood samples by effectively normalizing the
data using available DNA methylation signatures for major blood cell
types. Second, the authors use a clever series
of conditional correlation analyses involving genotype, methylation and
phenotype data to filter out differentially methylated positions (DMPs) that
are not likely to be causally related to RA.
Remarkably, this revealed significant associations between a set of SNPs
and DMPs located in the MHC gene cluster, which has previously been linked to
rheumatoid arthritis. In a final step,
the authors used a causal inference test to define 9 DMPs that mediate the
genetic risk for RA through interactions with 264 SNPs in the MHC region and
one SNP-DMP pair outside of the MHC region.
This
study not only reveals the importance of understanding the relationships
between genetic and epigenetic factors in common diseases, but also establishes
a clear methodology to overcome many of the issues inherent to EWAS studies.
Liu et al. Epigenome-wide association data implicate DNA
methylation as an intermediary of genetic risk in rheumatoid arthritis. Nature Biotechnology, published online
January 2013
Thursday, January 24, 2013
Retrieve SNPs in Promoters and Flanking Sequence for Many Genes
This post presents R code to retrieve SNPs in promoters for a list of genes. You provide your list of genes to the "gene" variable and then use biomaRt (mus_musculus) to get the transcriptional start sites (TSS) for each transcript for your list of genes. The code then uses the TSS info to search in promoter regions (defined here as [-1000, +200 bp] relative to TSS) for SNPs for each gene using biomaRt - my code looks for SNPs distinguishing C57BL/6J and CastEiJ mouse strains, but this can be easily altered in the getSnps function by changing "sp$cast_eij" to another strain name (use listAttributes(snpmart) in biomaRt).
You can view the promoters found to have SNPs in the "dataSnps" variable. Select the transcript SNP set you are interested in and run the final "getflank" function to get the surrounding sequence information using the mouse genome data provided in the BSgenome library. The code finds 100 bp of flanking sequence around each SNP site and this can adjust with the "offset" variable in "getflank" function. The "final" output provides row names and writes a tab delimited file that opens easily in Excel.
This is a quick way to get SNP data in promoter regions for genes of interest.
library(biomaRt)
library(BSgenome.Mmusculus.UCSC.mm10)
setwd("")

#######################INPUT GENES OF INTEREST####
genes = c("Igf2","H19", "Igf2R", "Rasgrf", "Magel2")


#######################GET TSS#############################
#get transcriptional start sites for all genes of interest

ensembl = useMart("ensembl")
ensembl = useDataset("mmusculus_gene_ensembl", mart=ensembl)
tss <- getBM(attributes=c('ensembl_gene_id', 'ensembl_transcript_id', 'chromosome_name','transcript_start', 'transcript_end','mgi_symbol'), filters = c("mgi_symbol"), values=genes, mart=ensembl)

########################GET SNPS IN PROMOTER###########################
#get snps in promoter region : promoter region is defined as [-1000,+200] relative to transcriptional start site

snpmart = useMart("snp")
snpmart = useDataset("mmusculus_snp", mart=snpmart)

getSnps <- function(x){
    txstart = as.numeric(x[4])
    txend = as.numeric(x[5])
    id = x[1]
    txid = x[2]
    name = x[6]
    chr = x[3]
    if ( txstart > txend ) {
        getBM(attributes=c('refsnp_id', 'chr_name', 'chrom_start', 'allele', 'c57bl_6j', 'cast_eij'), filters=c("chr_name", "chrom_start", "chrom_end"), values=list( chr, (txstart - 200), (txstart + 1000)), mart = snpmart)->sp
        sp[sp$cast_eij %in% c("A","T","G","C"), ]->dataSnps

        }    else if ( txstart < txend ) {
        getBM(attributes=c('refsnp_id', 'chr_name', 'chrom_start', 'allele', 'c57bl_6j', 'cast_eij'), filters=c("chr_name", "chrom_start", "chrom_end"), values=list( 2, ( txstart - 1000 ), ( txstart +200 )), mart = snpmart)->sp
        sp[sp$cast_eij %in% c("A","T","G","C"), ]->dataSnps
        }
    if ( nrow(dataSnps) > 1 ) {
    cbind(id,txid,name,dataSnps, txstart)->results
    return(results)
    }
}

snps<-apply(tss, 1, getSnps)
dataSnps <- snps[!sapply(snps, is.null)]#All SNP Info with NULLS removed

###########################GET FLANKING SEQUENCE FOR EACH SNP###########################
#Get sequence for snps

dataSnps #view output

dataSnps[[19]] -> d #select SNP set for transcript of interest

getflank <- function(x) {
    id = x[1]
    txid = x[2]
    name = x[3]
    position = as.numeric(x[6])
    alleles = paste("[",x[7]," > ",x[9],"]", sep="")
    chr = paste("chr", x[5], sep="")
    txstart = x[10]
    offset = 100
    leftflank  <- getSeq(BSgenome.Mmusculus.UCSC.mm10,chr,position-offset,position-1)
    rightflank <- getSeq(BSgenome.Mmusculus.UCSC.mm10,chr,position+1,position+offset)
    paste(leftflank,alleles,rightflank,sep="")->seq
    cbind(id, txid, name, txstart, position, alleles, chr, seq)->out
    return(out)
}


final <- apply(d, 1, getflank)
r<- c("id","txid", "name", "txstart", "snp position", "Ref > Alt", "chr", "Seq")
rownames(final) <- r
write.table(final, file = "SNPSandFlankingSEQinPROMOTERS_Gene.txt", sep="\t")
Monday, December 17, 2012
New Approaches to Gene Co-expression Network Analysis
 An important new paper on the methodology for doing gene co-expression network analysis was recently published in PLoS ONE by Kumari et al. (2012). The paper is entitled "Evaluation of Gene Association Methods for Coexpression Network Construction and Biological Knowledge Discovery".
The authors perform a comparative analysis of several different approaches for constructing co-expression networks.
____________________________________________________
Abstract:
Constructing coexpression networks and performing network analysis using large-scale gene expression data sets is an effective way to uncover new biological knowledge; however, the methods used for gene association in constructing these coexpression networks have not been thoroughly evaluated. Since different methods lead to structurally different coexpression networks and provide different information, selecting the optimal gene association method is critical.
Methods and Results: In this study, we compared eight gene association methods – Spearman rank correlation, Weighted Rank Correlation, Kendall, Hoeffding’s D measure, Theil-Sen, Rank Theil-Sen, Distance Covariance, and Pearson – and focused on their true knowledge discovery rates in associating pathway genes and construction coordination networks of regulatory genes. We also examined the behaviors of different methods to microarray data with different properties, and whether the biological processes affect the efficiency of different methods.
Conclusions: We found that the Spearman, Hoeffding and Kendall methods are effective in identifying coexpressed pathway genes, whereas the Theil-sen, Rank Theil-Sen, Spearman, and Weighted Rank methods perform well in identifying coordinated transcription factors that control the same biological processes and traits. Surprisingly, the widely used Pearson method is generally less efficient, and so is the Distance Covariance method that can find gene pairs of multiple relationships. Some analyses we did clearly show Pearson and Distance Covariance methods have distinct behaviors as compared to all other six methods. The efficiencies of different methods vary with the data properties to some degree and are largely contingent upon the biological processes, which necessitates the pre-analysis to identify the best performing method for gene association and coexpression network construction.
Sunday, December 9, 2012
Dr. Coni Horndli Receives Prestigious Swiss Fellowship!!
 Dr. Coni Horndli has been awarded a prestigious fellowship from the Swiss National Science Foundation. Dr. Horndli is a postdoctoral fellow in the Gregg Lab developing novel approaches to study genetic and epigenetic pathways in the brain that modulate complex feeding and foraging behaviors. She has a particular interest in molecular mechanisms that influence stress and anxiety. Dr. Horndli's work is anticipated to transform our understanding of the mechanisms in the brain that contribute to susceptibility to eating disorders, stress and anxiety-related disorders, and depression.
Wednesday, December 5, 2012
IGF2:IGF2R Evolution

By: Dr. Coni Horndli
An Exon Splice Enhancer Primes
IGF2:IGF2R Binding Site Structure and Function Evolution
Christopher Williams,1* Hans-Jürgen
Hoppe,2* Dellel Rezgui,2 Madeleine Strickland,1 Briony E. Forbes,3 Frank
Grutzner,3 Susana Frago,2 Rosamund Z. Ellis,1 Pakorn Wattana-Amorn,1 Stuart N.
Prince,2 Oliver J. Zaccheo,2 Catherine M. Nolan,4 Andrew J. Mungall,5 E. Yvonne
Jones,6 Matthew P. Crump,1† A. Bassim Hassan2†
ABSTRACT
Placental development and genomic
imprinting coevolved with parental conflict over resource distribution to
mammalian offspring. The imprinted genes IGF2 and IGF2R code for the growth
promoter insulin-like growth factor 2 (IGF2) and its inhibitor, mannose
6-phosphate (M6P)/IGF2 receptor (IGF2R), respectively. M6P/IGF2R of birds and
fish do not recognize IGF2. In monotremes, which lack imprinting, IGF2
specifically bound M6P/IGF2R via a hydrophobic CD loop. We show that the DNA
coding the CD loop in monotremes functions as an exon splice enhancer (ESE) and
that structural evolution of binding site loops (AB, HI, FG) improved therian
IGF2 affinity. We propose that ESE evolution led to the fortuitous acquisition
of IGF2 binding by M6P/IGF2R that drew IGF2R into parental conflict; subsequent
imprinting may then have accelerated affinity maturation.
COMMENT
This report published by Matthew
Crump’s and Bassim Hassan’s groups this week in Science analyses the
evolutionary molecular changes, which led to high affinity binding of IGF2R to
IGF2 in mammals but not birds and reptiles. IGF2 and IGF2R are two of the
roughly 100 canonically imprinted genes found in mammals, with IGF2 expressed
only from the paternal allele and IGF2R only from the maternal allele. In mice,
deletion of the maternal IGF2R gene results in overly large offspring while deletion
of the paternal IGF2 gene results in dwarf offspring. In humans, only IGF2 is
imprinted but not its receptor. Activation of the maternal IGF2 allele causes
Beckwith-Wiedemann syndrome, which is characterized large body size at birth
and an increased risk for childhood cancer. The reciprocal expression of IGF2
and IGF2R underscores the parental conflict over the distribution of resources
to their offspring. This hypothesis is based on the theory that mothers want to
distribute their resources equally to all their current and future offspring,
while fathers favor the maternal investment into the current offspring.
This study correlates the appearance of
IGF2/R with the occurrence of their monoallelic expression. Specifically,
Williams et al. show that binding appeared in all primitive mammals, while
imprinting is only found in theria, such as rodents, kangaroos and opossums.
Therefore, the authors hypothesize that the evolution of IGF2/R imprinting was
facilitated by the appearance of their molecular binding, which may conversely
have accelerated the selection for improved regulation of IGF2 through IGF2R.
This report thoroughly reveals the
structural changes that lead to IGF2:IGF2R complex formation but falls short on
explaining the mechanism of how IGF2/R binding facilitates genomic imprinting
of these two genes.
Innovator of the Year 2012 - Sridhar Vukkadapu
2012 Innovator of the Year Award
The 2012 Gregg Lab Innovator of the Year is Sridhar Vukkadapu. Sridhar is completing his Master's Degree in computer science and has worked in the lab for one year. He has developed a software pipeline for the analysis of allele-specific gene expression using high-throughput sequencing. The pipeline, called PARENT SEQ'R, is a full suite of code written in C++, Python, Perl and Processing that manages the alignment, processing, analysis and visualization of RNA-Seq data to study allele-specific gene expression. It is a tour de force achievement that opens up new ways of studying gene expression data and has revealed many new discoveries in the lab. We look forward to making the pipeline and data visualization software publicly available in the future following publication!!
Thursday, November 15, 2012
Identification of Neurons Regulating Energy Expenditure
By: Dr. Coni Horndli PhD.
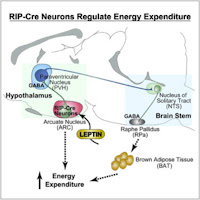
This recent study in Cell from Brad Lowell's group reveals novel circuits in the arcuate nucleus of the hypothalamus that selectively drive energy expenditure. The authors integrate genetic and
electrophysiological approaches with studies of metabolism and neuronal circuit
mapping to reveal a defined population of GABAergic neurons that regulate brown fat and energy expenditure. It remarkable to see such potent neural control over these aspects of physiology.
The authors use an elegant double-labeling method to reveal functional
neuronal connectivity between RIP-Cre ARC - PVH - NTS neurons. First, a
Cre-dependent virus, which expresses a channelrhodopsin-mCherry fusion protein
(AAV-Flex-ChR2(H134R)-mCherry) was stereotaxically injected in the ARC of RIP-Cre
mice. Second, retrograde green fluorescent beads were injected into the NTS of
the same mice. Electrophysiological recordings specifically showed light-evoked
IPSCs in bead+ PVH neurons.
In this study, a synthetic receptor was expressed in RIP-Cre mice and
activated by the pharmacological compound CNO. Neuronal activity in response to
CNO and later leptin were recorded in cultured brain slices. It would be
interesting to see whether the same neuronal responses can be elicited using an
in vivo approach.
In the ARC, only 30% of RIP-Cre neurons showed an excitatory response to
leptin, while 35% of ARC RIP-Cre neurons were inhibited. If and how ARC neurons
exhibiting these differential responses integrate into one circuit and or what
the role of leptin-inhibited ARC RIP-Cre neurons is in regulating energy
expenditure is not clear at this point. Also, I am wondering how, where and
when AgRP, which reside in the ARC, project to the PVH and are also GABAergic
but inhibit energy expenditure and food intake interplay in the RIP-Cre ARC -
PVH - NTS circuitry.
REFERENCE AND ABSTRACT:
GABAergic RIP-Cre Neurons in the Arcuate Nucleus Selectively
Regulate Energy Expenditure
Dong Kong, Qingchun Tong,
Chianping Ye, Shuichi Koda,
Patrick M. Fuller, Michael
J. Krashes, Linh Vong,
Russell S. Ray, David
P. Olson, and Bradford B. Lowell
SUMMARY
Neural
regulation of energy expenditure is incompletely understood. By genetically
disrupting GABAergic transmission in a cell-specific fashion, and by combining
this with selective pharmacogenetic activation and optogenetic mapping
techniques, we have uncovered an arcuate-based circuit that selectively drives
energy expenditure. Specifically, mice lacking synaptic GABA release from
RIP-Cre neurons have reduced energy expenditure, become obese and are extremely
sensitive to highfat diet-induced obesity, the latter due to defective diet
induced thermogenesis. Leptin’s ability to stimulate thermogenesis, but not to
reduce feeding, is markedly attenuated. Acute, selective activation of arcuate
GABAergic RIP-Cre neurons, which monosynaptically innervate PVH neurons
projecting to the NTS, rapidly stimulates brown fat and increases energy
expenditure but does not affect feeding. Importantly, this response is
dependent upon GABA release from RIP-Cre neurons. Thus, GABAergic RIP-Cre neurons
in the arcuate selectively drive energy expenditure, contribute to leptin’s
stimulatory effect on thermogenesis, and protect against diet-induced obesity.
|
|


Thursday, November 1, 2012
Nematocin; identification of a C. elegans peptide neurotransmitter with structural and functional homology to vertebrate vasotocin and vasopressin/oxytocin.
By: Dr. Paul Bonthuis PhD.
 Two simultaneous reports by Garrison et al. and Beets et al. in last week's issue of Science discovered a C. elegans peptide neurotransmitter, and two cognate receptors, with genetic, structural, and functional similarity to the mammalian oxytocin/vasopressin (and non-mammalian vertebrate vasotocin) signaling systems. In mammals, oxytocin and vasopressin are structurally similar octomeric neuropeptides that are secreted from the pituitary and have wide ranging effects on physiology and complex behaviors, including many social behaviors. For example, these molecules have been linked to pair-bonding and monogamous behaviors in voles. Amazingly, similar to the roles of oxytocin/vasopressin, the 11-mer C. elegans peptide "neurotocin", and the genes for the receptors ntr-1 and ntr-2, display sexually dimorphic expression in the C. elegans nervous system and were proved to play important roles in reproductive and learned foraging behaviors of the worm. The finding of an ancient neural regulator in the structurally simple nervous system of the worm that has conserved functional roles on behavior with the structural complex nervous systems of vertebrates, has the potential to reveal fundamental mechanistic insights on the neural regulation of complex behaviors. For a thorough explanation of the implications of the discoveries, read "The Mood of the Worm" by Scott Emmons in the same issue of Science.
REFERENCES and ABSTRACTS:
Science 26 October 2012:
Vol. 338 no. 6106 pp. 540-543
DOI: 10.1126/science.122620
Oxytocin/Vasopressin-Related Peptides Have an Ancient Role in Reproductive Behavior
1. Jennifer L. Garrison,
2. Evan Z. Macosko,
3. Samantha Bernstein,
4. Navin Pokala,
5. Dirk R. Albrecht,
6. Cornelia I. Bargmann
Abstract
Many biological functions are conserved, but the extent to which conservation applies to integrative behaviors is unknown. Vasopressin and oxytocin neuropeptides are strongly implicated in mammalian reproductive and social behaviors, yet rodent loss-of-function mutants have relatively subtle behavioral defects. Here we identify an oxytocin/vasopressin-like signaling system in Caenorhabditis elegans, consisting of a peptide and two receptors that are expressed in sexually dimorphic patterns. Males lacking the peptide or its receptors perform poorly in reproductive behaviors, including mate search, mate recognition, and mating, but other sensorimotor behaviors are intact. Quantitative analysis indicates that mating motor patterns are fragmented and inefficient in mutants, suggesting that oxytocin/vasopressin peptides increase the coherence of mating behaviors. These results indicate that conserved molecules coordinate diverse behavioral motifs in reproductive behavior.
Science 26 October 2012:
Vol. 338 no. 6106 p. 469
DOI: 10.1126/science.1225996
Vasopressin/Oxytocin-Related Signaling Regulates Gustatory Associative Learning in C. elegans
1. Isabel Beets1,
2. Tom Janssen1,
3. Ellen Meelkop1,*,
4. Liesbet Temmerman1,
5. Nick Suetens1,
6. Suzanne Rademakers2,
7. Gert Jansen2,
8. Liliane Schoofs1,†
Abstract
Vasopressin- and oxytocin-related neuropeptides are key regulators of animal physiology, including water balance and reproduction. Although these neuropeptides also modulate social behavior and cognition in mammals, the mechanism for influencing behavioral plasticity and the evolutionary origin of these effects are not well understood. Here, we present a functional vasopressin- and oxytocin-like signaling system in the nematode Caenorhabditis elegans. Through activation of its receptor NTR-1, a vasopressin/oxytocin-related neuropeptide, designated nematocin, facilitates the experience-driven modulation of salt chemotaxis, a type of gustatory associative learning in C. elegans. Our study suggests that vasopressin and oxytocin neuropeptides have ancient roles in modulating sensory processing in neural circuits that underlie behavioral plasticity.
Wednesday, October 12, 2011
NYSCF-Robertson Neuroscience Investigator

In addition to Christopher Gregg, the neuroscience winners this year include:
Ed Boyden: A pioneer in the field of optogenetics at MIT.
Takaki Komiyama: A pioneer in the use of two-photon imaging to study neuronal activity and motor learning in the brain of awake behaving animals at UCSD.
Gaby Maimon: A leader in the development of approaches to record neuronal activity in awake and behaving fruit flies to uncover neural processes regulating decision making. He is located at Rockefeller University.
Big thanks to NYSCF and all of the great people who support this powerful initiative!
Learn more here: New York Stem Cell Foundation
Friday, July 29, 2011
Writing a Research Proposal - Quick Tips

Great science writing might be described as a strange form of poetry that brings beautiful ideas to life with piercing clarity and purpose. Getting good at this is a career long endeavour. PhD students write for awards, for preliminary exams and for manuscripts to be published. Postdocs write for journal manuscripts, fellowships, awards, and ultimately, their own grants! Professors write for everything from grants to journal manuscripts to textbooks. Write…write…write. Communication is a central component of a science career. This article is about how to write a research proposal, which is often done to get money from funding agencies, and is therefore, very important. Here, I include useful tips I have gathered from experienced and successful colleagues.
A Basic Outline for a Five Page Research Proposal
Some General Comments:
Your proposal must present a great idea to address an important and interesting problem. Be Original. Focus the proposal on one clear central problem such that the Aims logically work towards addressing that central problem and the whole proposal logically adheres to a major theme. Break each aim into separate goals that address the proposed aim. For each goal, clearly lay out (1) the Rational (background logic), (2) the Problem (what is not known), (3) the Approach (how you will solve the problem), (4) What you expect to learn and why it is significant, (5) A final transition sentence that logically prepares the reader for the next goal or aim. Whenever possible/appropriate, emphasize some unique strength or expertise you have that will set you up to achieve what you are proposing and convince the reader you are the person for the job!
DO NOT EXCEED THE MAXIMUM PAGE LENGTH BY EVEN ONE SENTENCE - KEEP IT TIGHT. Do not shrink fonts or margins that might make it more of a strain to read. Do not repeat yourself. Do not repeat yourself. Introduce ideas and supporting studies strategically, such that they appear in the context that they are the most effective. For example, don't introduce an idea in the introduction that is specifically meant to set up an experiment in Aim 3.
Assume readers will not make any intellectual leaps on your behalf. Therefore, clearly explain what you are proposing and why you are proposing it throughout the grant. Above all keep it simple. Note that excessive detail will disrupt the flow, the logic and the excitement and will expose you to criticism. Strategically use italics and underlining to highlight key points and steer the reader's attention throughout the text of the proposal - make it easy for the reader to find the important information. I tend to save bold print for titles.
Number your aims and goals to maintain a logical organization.
In many ways, a truly great research proposal can take years of thought, planning, experimentation and pruning. I keep a database of ideas and I am constantly developing new research programs that could be grants. Many good ideas get rejected in order to focus on a core idea. You MUST get feedback from colleagues and in my experience your first draft should be completed 4 weeks prior to the deadline to allow you to really nail it!!! It takes that long to go through internal reviews and develop corrected drafts with busy colleagues. So plan ahead.
Finally, I believe that humans fundamentally understand things in terms of stories and good stories have a particular structure and feel. Your proposal is a story about an idea, a discovery or a deep desire to understand something fundamental and potentially transformative. Inject your prose with that active feeling of excitement, because that is what you want your readers to feel. Do NOT use a passive voice in the writing.
Write a long draft and then start working on the poetry to polish it and get it within the size limits…
_______________________________________
1. Title:
Must be brief, snappy, informative and interesting. Beware of including buzz words that will bury your proposal in the pile of others doing similar work. Find a title that encapsulates the main themes and most unique aspects of your research proposal. Be original. Avoid boring words like "Characterization of..." or "Investigation into…". Get feedback!
In addition, if it is appropriate, I like to put a picture on the title page. It can be a schematic or artistic image. Something that speaks to the central theme and will help the proposal standout from the stack of competing papers. People are visual creatures and a nice image is eye catching.
2. Abstract (1 paragraph):
This is a make it or break it section. It has to be crisp, concise and have punch. It needs to express: (1) The rational for the study, (2) The central problem to be addressed in the study ("Based on these new data, I propose to investigate…"), (3) Clearly state the specific aims that will address the central problem ("I will pursue the following three aims: (1) …, (2) …, and (3) … "). I usually present the aims in bold print, so they standout. (4) One sentence that summarizes the significance and potential impact of the work.
3. Introduction (2 paragraphs):
In general, describe the published works that have revealed the central problem of interest. Your first sentence must immediately communicate the big picture importance and context of the work. The introduction includes information that builds the logical foundation of your proposal by drawing from previous work and different disciplines to bring together a new, coherent and exciting direction for your field. You likely do not want to beat an old horse by rehashing logical, but well studied research directions that everyone is pursuing and publishing on. Novelty must shine through. Exclude any extra information that does not logically flow toward your central problem of interest, and may therefore distract the reader. In the final sentence of the introduction, clearly and concisley state the central problem that arises from the work described and cited or at least provide a summary statement with a logical link to the Background section.
4. Background (1 paragraph):
Use this section to describe what you have done thus far to bring you to this problem. Did you discover something? What? Have you developed some new approach? What is it? You need to sell the idea that no one is better than you to address the problem built up in the Abstract/Intro through the studies that will be proposed. Also use this section to clarify supporting and opposing evidence for your previous findings. In the final two sentences of the background, highlight the major questions that have arisen as a result of your work and clearly and concisley state the direction of your study. Keep the logical flow of the abstract and introduction. This is a good section for a figure that highlights an important and very interesting aspect of your previous work.
5. Specific Aims:
Typically, a grant/research proposal has 3 specific aims. Specific aims should be stand alone projects that are interrelated, but not interdependent. Ask yourself, what happens if Aim 1, 2 or 3 fails - will it take the whole proposal down with it? Each aim must be fantastically important and interesting in its own right. Ideally, an aim should look contain a logical project that one can imagine a student or postdoc carrying out.
Each aim is subdivided into specific goals that clearly indicate a particular problem to be solved to achieve the aim. Each goal is 1-2 paragraphs. For each goal, include the following information:
1. The rational for this goal (2 sentences).
2. The problem to be solved (1 sentence).
3. The approach that will be used to solve the problem (experimental design).
4. The potential findings and impact of these findings (1-2 sentences).
5. Where to next? Include a final transition sentence to flow logically into the next goal or aim (1 sentence).
Titles for aims and goals should be considered carefully. Words like "Characterize…", "Investigate…", Explore…", "Identify…" or "Study…" can be construed as proposing fishing expeditions, though they may be appropriate. When possible, a clear statement that flows from a hypothesis is preferred and words like "Determine whether…" or "Test the hypothesis that…" can be more powerful and direct.
6. Figures:
Embed simple figures in the text that present provocative preliminary findings. Insert them directly into the text and use the text wrap tool in Word. Write a short caption underneath by inserting a text box. The font for figure legends can be smaller than the main text 12 point minimum. The figures must be thought provoking and support the central questions and approaches posed in the grant. These figures need to strategically address potential sticky points by illustrating complex ideas or by revealing that your ideas are on the right track. In addition, they should present stuff that gets reviewers thinking about the possibilities of your proposal. Give them a chance to imagine how big this idea could be, so they get excited! Less is often more. Don't make the figures to complicated, just thought provoking seeds.
7. Timeline (indicate in brackets with aims and goals or provide bulletin points in a separate 'Timeline' section):
Reviewers need to known when specific aspects of your proposal will be initiated during the funding period and how long you think they will take to complete. Based on this information they will decide if you have proposed a project that reasonably fits with the timeline of the funding period.
8. Significance (1 paragraph):
Use this final section to first clarify the big idea you are proposing. Next, address how the results will be transformative conceptually. Address the potential impact on the field. Finally, address the potential impact for human health and wellbeing. Be concise and clear about what will come from the study. As always, if you are vague and descend into buzz words, the impact of this section will be lost. The reviewers really want to known exactly what you expect to find, so tell them and be clear about why you think it will be awesome. Thinking a lot about this section can help you clarify in your mind what the central importance of your study really is.
Other Resources:
Friday, May 27, 2011
ReExamining Lab Rotations - What should this graduate training experience be about?

One of the first steps in graduate school is to figure out what you want to study and in which lab you want to do your research. Lab rotations typically involve working in ~3 different labs for 1-2 months each. The experience provides students an opportunity to shop around a little and the PIs get some insight into which students might fit best in with their group. Fundamentally, this is a reasonable idea. In practice however, it is a bit of muddled scramble. In my time as a postdoc at Harvard, I saw lots and lots of rotation students come through. The time they spend in the lab is short and they are not yet trained, so their projects are simple and they really cannot see anything through to completion. The simple projects they tend to get are sometimes tedious and repetitive. While this is the nature of experimentation, as a first experience, it fails to engage the imagination. What can be done to improve the rotation experience?
One perspective is to accept that short rotations generally fail to generate useful data and let go of the idea of trying to get a big result or start a thesis project. Instead, the PI might select a few specific observational experiments that have no point other than to engage the imagination and generate questions and ideas.
In the Gregg Lab, for example, a rotation experience would ideally expose an individual to major questions and ideas related to: (1) gene expression and bioinformatics, (2) feeding circuits, (3) early life programming, and, (4) feeding and foraging behaviors. For a four week rotation, each week would be committed to one of these four topics. A student would carry out an experiment that is short term and very likely to work, and most importantly, leads to lots of opportunity for observation and thought. To guide the thinking and discovery process, I have taken some ideas from Tim Hurson's useful book, 'Think Better', and generated a simple outline that provides rotation students with a framework to conceptually explore the potential of their data (see Project Planner). The key is to push yourself to think deeply about what you are observing. The first round of ideas that come to you will likely be ones that others have considered, but by the time you push yourself to a third round of ideas you may be starting to come up with original material.
Consider that a simple immunohistochemical stain of neural circuitry in the brain can illuminate a million questions and ideas. A simple study of animal behavior can force one to reflect on all of the problems the brain must solve to carry out a task and wonder what behaviors the animal is capable of. A brief bioinformatic study of gene interactions and expression patterns raises numerous questions about how everything works. The point of the rotation experience is to engage your mind and find a topic that is exciting and important to you and demonstrate to the PI that you are an independent thinker!
Subscribe to:
Posts (Atom)